The Michaelis–Menten equation describes how the rate of an enzyme-catalysed reaction increases with substrate concentration and eventually plateaus at a maximum value (\(v_{max}\)) due to enzyme saturation.
Consider an enzyme \(E\) binding reversibly to a substrate \(S\) to form the Michaelis complex \(ES\), which then produces product(s) \(P\) and regenerates the enzyme:
$$E+S\overset{k_{1}}{\underset{k_{-1}}{\rightleftharpoons}}ES\xrightarrow{k_2} E + P$$
where \(k_1\), \(k_{-1}\) and \(k_2\) are rate constants.
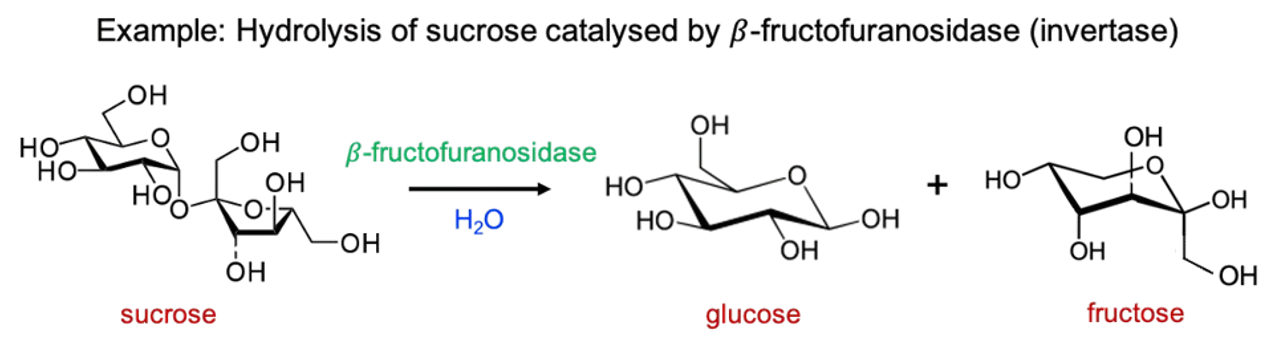
The rate of formation and breakdown of \(ES\) is given by:
$$\frac{d[ES]}{dt}=k_1[E][S]-(k_{-1}+k_2)[ES]$$
Let’s assume:
-
- The initial rate method is used to measure the reaction.
- The initial substrate concentration \([S]_0\) is much greater than the initial enzyme concentration \([E]_0\), so that the free substrate concentration \([S]\) is approximately equal to \([S]_0\).
- Initial product formation is negligible and the step \(ES\rightarrow E+P\) is irreversible.
- Total enzyme concentration is conserved: \([E]_0=[E]+[ES]\).
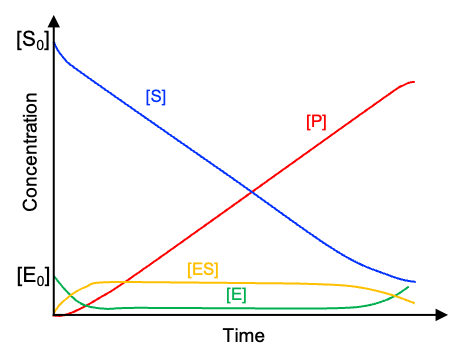
Therefore, the enzyme–substrate complex builds up rapidly during an initial transient phase and then reaches a constant concentration (see diagram above). During this period, \(\frac{d[ES]}{dt}=0\). This is known as the steady-state approximation, with
$$\frac{[E][S]}{[ES]}=K_M\;\;\;\;\;\;\;\;80$$
where \(K_M=\frac{k_{-1}+k_2}{k_1}\) is the Michaelis constant.
Substituting \([E]=[E]_0-[ES]\) into eq80 gives:
$$[ES](K_M+[S])=[E]_0[S]$$
which rearranges to:
$$[ES]=\frac{[E]_0}{1+K_M/[S]}$$
Since \([S]\approx [S]_0\),
$$[ES]=\frac{[E]_0}{1+K_M/[S]_0}\;\;\;\;\;\;\;\;81$$
Because product formation is relatively slow initially, \(ES\rightarrow E+P\) becomes the rate determining step, with the initial reaction velocity \(v\) of the overall reaction being:
$$v=\frac{d[P]}{dt}=k_2[ES]\;\;\;\;\;\;\;\;82$$
Substituting eq81 into eq82 yields the Michaelis-Menten equation:
$$v=\frac{v_{max}}{1+K_M/[S]_0}\;\;\;\;\;\;\;\;83$$
where \(v_{max}=k_2[E]_0\) is a constant for a fixed \([E]_0\).
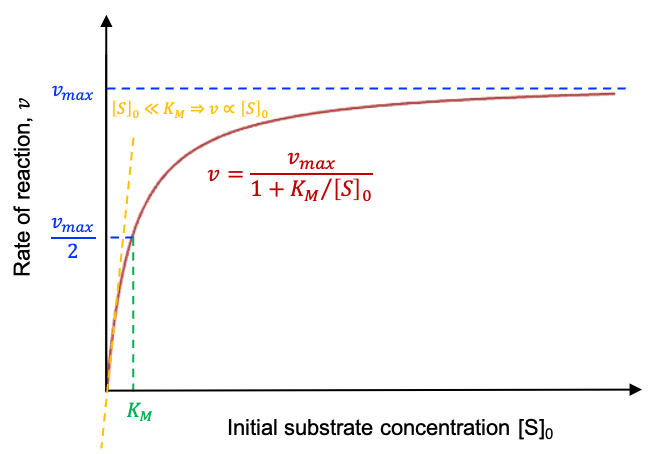
When \([S]_0\gg K_M\), we have \(v\approx v_{max}\) (see above diagram). In other words, the rate of the enzyme-catalysed reaction reaches a maximum when the substrate concentration is in excess. Here, the reaction is zero-order with respect to the substrate concentration.
Rearranging eq83 to \(v=\frac{v_{max}[S]_0}{[S]_0+K_M}\) shows that at low initial substrate concentration (\([S]_0\ll K_M\)), the reaction approximates first-order kinetics for a fixed \([E]_0\): \(v=\frac{v_{max}}{K_M}[S]_0\propto [S]_0\).
When \([S]_0=K_M\), we have \(v=\frac{1}{2}v_{max}\).
At a specific temperature and pH, \(K_M\) is characteristic for a given enzyme-substrate pair. It can be interpreted as a measure of the affinity of the enzyme for its substrate because it can be rewritten as:
$$K_M=K_S+\frac{k_2}{k_1}$$
Here, \(K_S=\frac{k_{-1}}{k_1}\) is the equilibrium constant for \(ES\rightleftharpoons E+S\). A smaller \(K_S\) (and hence a smaller \(K_M\)) corresponds to greater the affinity of the enzyme for its substrate, since the enzyme–substrate complex is less likely to dissociate back into free enzyme and substrate. Additionally, because \(K_M\) is equal to the substrate concentration at which the reaction rate is half-maximal, a smaller \(K_M\) means the enzyme can achieve this rate at lower substrate concentrations and therefore operates more efficiently.
Question
What is the definition of catalytic efficiency?
Answer
Catalytic efficiency is defined as \(\frac{v_{max}}{[E]_0K_M}\), which is equivalent to \(\frac{k_2}{K_M}\) because \(v_{max}=k_2[E]_0\). The term \(\frac{v_{max}}{[E]_0}\) corresponds to the maximum number of reactions each enzyme molecule can catalyse per unit time. Furthermore, a smaller \(K_M\) indicates a higher affinity of the enzyme for its substrate. Therefore, \(\frac{v_{max}}{[E]_0K_M}\) captures both the catalytic speed and substrate-binding efficiency of the enzyme, with a larger value indicating higher catalytic efficiency.
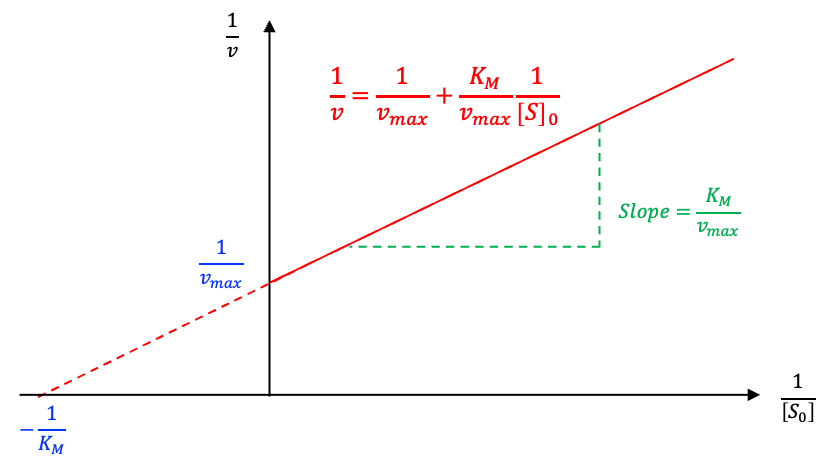
To determine \(K_M\) experimentally, \(v=\frac{v_{max}[S]_0}{[S]_0+K_M}\) is rearranged into a Lineweaver-Burk form:
$$\frac{1}{v}=\frac{1}{v_{max}}+\frac{K_M}{v_{max}}\frac{1}{[S]_0}$$
A plot of \(\frac{1}{v}\) against \(\frac{1}{[S]_0}\) for different initial substrate concentrations results in a straight line with intercept \(\frac{1}{v_{max}}\) and slope \(\frac{K_M}{v_{max}}\), from which \(K_M\) can be determined (see diagram below).